Animals and plants use conceptually similar immune systems to detect microbes and activate defenses. In both lineages, pattern recognition receptors (PRRs) perceive pathogen- or microbe-associated molecular patterns (PAMPs or MAMPs) and host-derived damage-associated molecular patterns (DAMPs). Whereas animals rely on specialized immune cells, plants harness individual cells expressing diverse PRRs. In the apoplast, which lies outside the plasma membrane and includes the cell wall, PRRs detect immunogenic fragments released from microbial proteins by plant hydrolytic enzymes. Conversely, pathogen-secreted enzymes can degrade constituents of the apoplast, generating DAMPs that activate immunity.
Three independent articles published on page 298, 291, and 290 respectively of this issue of the Science issue of October 15th, 2026 report expansion of this surveillance, revealing receptor architectures and mechanisms, that enable plants to discriminate immunogenic carbohydrates.
Gysel et al. identify a chitin perception (CHIP) receptor from Lotus japonicus and Medicago truncatula that binds to long-chain chito-oligosaccharides. Jiménez-Sandoval et al. structurally and functionally characterized the plant receptor kinase IGP1 to understand how plants perceive these cell wall–derived glycans. Huang et al. identify an apoplastic protein as a chitosan receptor in rice called O. sativa fungal infection defender 1(OsFID1). This soluble receptor is a type of domain of unknown function 26 (DUF26) protein—carbohydrate-binding proteins that are specific to land plants./
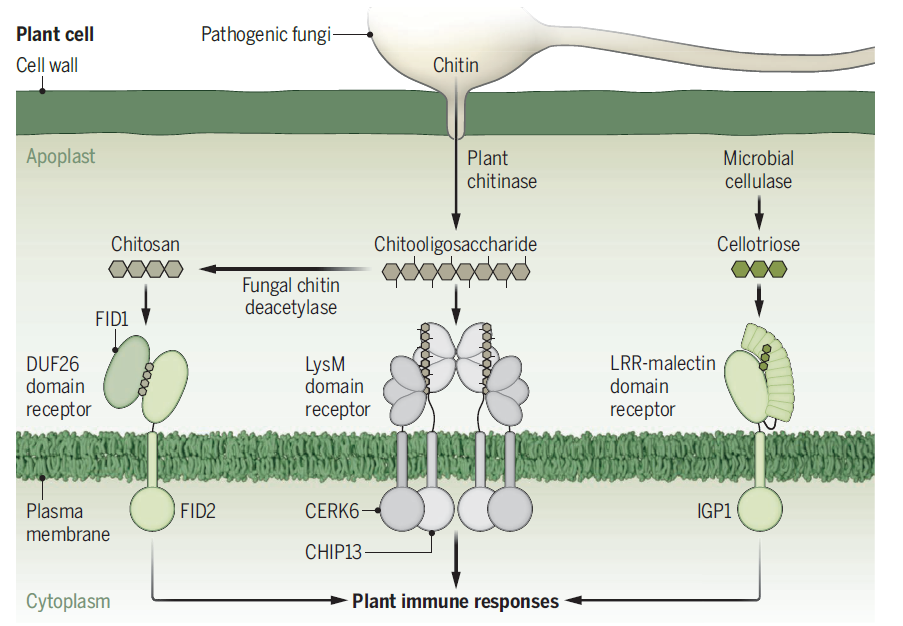
Figure: CERK6, chitin elicitor receptor kinase 6; CHIP13, chitin perception 13; DUF26, domain of unknown function 26; FID1 and FID2, fungal infection defender 1 and 2; IGP1, impaired in glycan perception 1; LRR, leucine-rich repeat; LysM, lysin motif.